 Sylva Botanical Journal
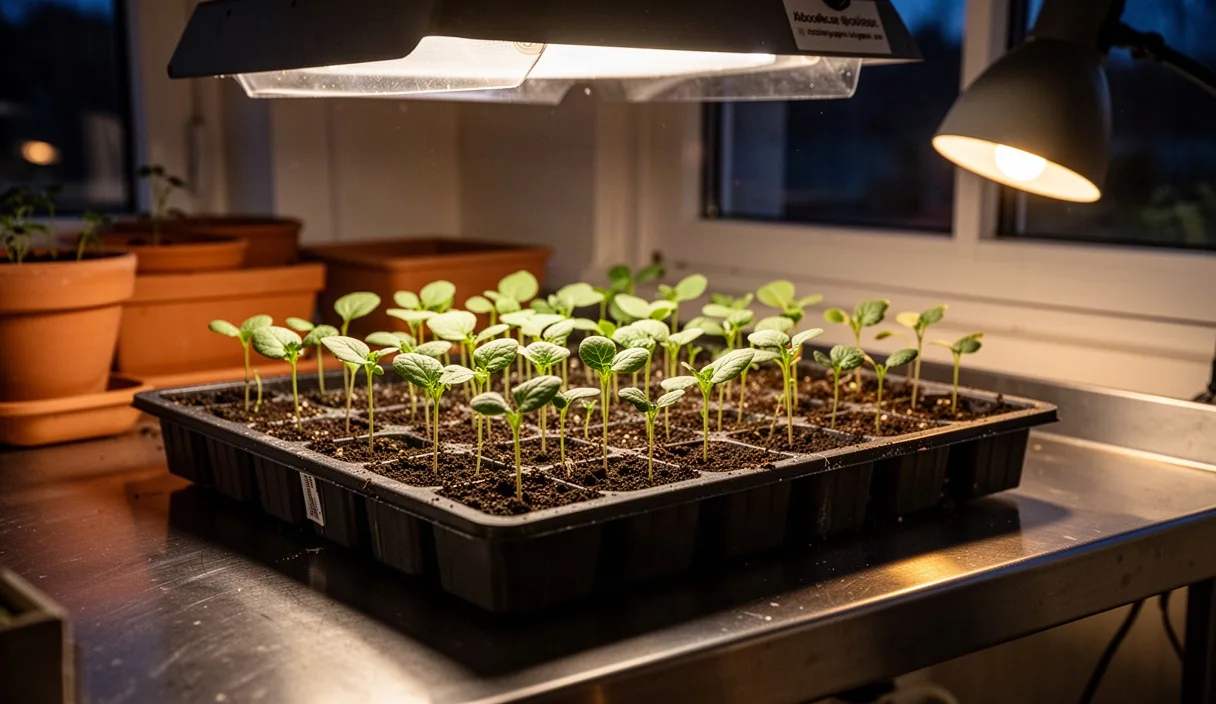
Closed-cycle germination chambers offer an unprecedented degree of environmental control, allowing propagation managers to isolate light spectra, modulate diurnal temperature curves, and conserve water within an insulated thermal shell. Yet this very isolation compounds the hazard of biological contamination. When fungal or oomycete spores settle into a recirculating environment devoid of weather fluctuations and natural UV radiation, the consequences are rarely limited to individual cell clusters. An entire crop of dormant native perennials or recalcitrant hardwood seedlings can disintegrate within thirty-six hours of emergence.
The condition broadly termed damping-off represents not a single malady, but a suite of symptomatic failures caused by distinct soil-borne and air-assisted organisms attacking tender embryonic tissue. Within sealed propagation vaults, where internal fans cycle warmed air over saturated trays, the line between vigorous germination and wholesale hypocotyl collapse is exceptionally thin. Cultivators who operate these systems cannot rely on casual sanitation; managing post-emergence decay requires an exact understanding of pathogen biology, rigorous thermodynamic balancing, and calculated hydration tactics.
Etiology of Common Post-Emergence Pathogens
Successful intervention requires distinguishing between true fungi and the fungus-like protists of the class Oomycota. The most pervasive culprit in saturated substrate is Pythium ultimum, alongside related species such as Pythium aphanidermatum. These oomycetes produce biflagellate zoospores that actively swim through free water film within macro-pores. In closed-loop systems with substrate moisture held near field capacity, Pythium targets the hypocotyl directly at the soil line, deploying pectolytic enzymes that liquefy host cell walls and turn the stem into a water-soaked, thread-like lesion.
In contrast, Rhizoctonia solani presents as a sterile fungus that does not form asexual spores under standard cultivation regimes, spreading instead through thick, brown vegetative hyphae that branch at distinctive ninety-degree angles. Unlike the water-loving oomycetes, Rhizoctonia thrives across a wider spectrum of moisture conditions, often attacking seedlings in drier substrates where the relative air humidity remains saturated. It typically forms dry, wire-stem cankers, girdling the plant just above the root crown and producing a characteristic toppling symptom where the foliage remains green even as the base rots.
Fungi belonging to the genera Fusarium and Phytophthora constitute secondary yet destructive agents. Fusarium oxysporum invades vascular bundles, leading to unilateral wilting, stunting, and root rot under warmer temperatures, frequently exceeding 26 degrees Celsius. Phytophthora species share the zoosporic mobility of Pythium but display greater destructive potential against woody taproots, persisting in organic debris as resilient chlamydospores or oospores capable of surviving long periods of fallow dormancy within plastic tray crevices.
| Pathogen | Organism Type | Primary Infection Vector | Optimal Temperature Range | Characteristic Stem Pathology |
|---|---|---|---|---|
| Pythium ultimum | Oomycete | Flagellated zoospores in free water | 15 to 20 degrees Celsius | Soft, translucent, water-soaked rot at soil interface |
| Rhizoctonia solani | Basidiomycete fungus | Vegetative hyphae from organic residues | 22 to 28 degrees Celsius | Sunken, dry, reddish-brown cortical lesions |
| Fusarium oxysporum | Ascomycete fungus | Microconidia in air, dust, and water lines | 25 to 30 degrees Celsius | Vascular discoloration, early petiole epinasty |
| Phytophthora cactorum | Oomycete | Zoospores and splash-dispersed sporangia | 18 to 24 degrees Celsius | Dark brown to black necrotic girdling extending upward |
Substrate Sterilization and Sanitation Protocols
Commercial peat, coir, and vermiculite blends are frequently marketed as sterile, yet transit, warehousing, and bulk handling regularly compromise their pristine state. For sensitive stratification seed lots, proprietary mixes must undergo thermal pasteurization or verified chemical remediation prior to tray loading. Thermal pasteurization requires aerated steam exposure that elevates substrate temperatures to 82 degrees Celsius, maintaining that threshold for precisely thirty minutes. Temperatures beyond 88 degrees Celsius risk releasing toxic concentrations of manganese and converting organic nitrogen into plant-toxic ammonium salts, while failing to clear the 71-degree barrier leaves durable resting spores of Rhizoctonia intact.
Reusable propagation trays and cell inserts present an equal vector risk. Simple high-pressure water washing leaves behind microscopic organic films inside root-guiding grooves. A thorough decontamination regime requires physical scrubbing followed by a soaking immersion sequence:
- Physical scrubbing with warm water and an agricultural detergent to dislodge root scale and mineral deposits.
- Immersion in an aqueous solution of peracetic acid and hydrogen peroxide at a dilution rate of 1:100 for twenty minutes, ensuring active effervescence contacts all corners.
- Alternatively, a prolonged immersion in a freshly prepared solution of sodium hypochlorite at a concentration of 0.6% available chlorine for a minimum of fifteen minutes, followed by a double rinse in reverse-osmosis water to strip residual chloride salts.
- Drying on slatted aluminum drying racks maintained under low-spectrum ultraviolet lighting to discourage dust accumulation before filling.
Chamber walls, internal circulation ductwork, and aluminum racking demand scheduled fumigation or cold fogging. Applying vaporized hydrogen peroxide via a specialized cold-aerosol generator ensures penetration into the micro-fissures of gaskets, blower impellers, and condensate drains where fungal spores accumulate undetected between stratification batches.
Air Circulation Dynamics and Vapor Pressure Deficit
The atmosphere inside a closed chamber rapidly approaches saturation without active psychrometric management. When air stagnates adjacent to the seedling canopy, transpiration stalls. A thick, motionless boundary layer forms over the hypocotyl and cotyledons, driving the localized relative humidity to near saturation regardless of broader room sensor readings. This boundary layer prevents the evaporation of guttation droplets, providing the moisture film that Pythium and Rhizoctonia spores require to germinate and penetrate the cuticle.
Modulating vapor pressure deficit, abbreviated as VPD, serves as the primary mechanical hedge against infection. The goal is to sustain a transpirational pull sufficient to move calcium to expanding leaf margins while avoiding tissue desiccation. For emergent seedlings, propagation chambers should operate within a VPD range of 0.8 to 1.1 kiloPascals. Maintaining this deficit requires balancing air temperature and relative humidity simultaneously; if air temperature rests at 21 degrees Celsius, relative humidity must remain between 68% and 74% to preserve adequate drying pressure at the boundary layer.
Horizontal laminar airflow prevents the formation of pocketed microclimates. Blower systems must produce an air velocity across the tray surface between 0.3 and 0.5 meters per second. Velocities below 0.2 meters per second allow the humid boundary layer to persist, whereas air speeds exceeding 0.7 meters per second cause mechanical stress, uneven drying of perimeter cells, and premature desiccation of newly emerged radicles. Gentle, continuous air movement also thickens stems through thigmomorphogenesis, building physical resistance against mechanical hyphal ingress.
Sub-Irrigation Versus Overhead Mist Regimens
Overhead spray nozzles remain a standard fixture in commercial horticulture, yet they are structurally ill-suited to closed-cycle chambers dedicated to damping-off management. Overhead misting wets the foliage, pools moisture at the base of the hypocotyl, and repeatedly washes fungal spores from the air column directly down into the root zone. Furthermore, droplet impact compacts the upper two millimeters of substrate, reducing oxygen diffusion and creating the exact anoxic, saturated surface conditions under which oomycete zoospores thrive.
Sub-irrigation regimens, managed via ebb-and-flow tables or automated capillary troughs, present an effective countermeasure. By introducing water exclusively from the base of the cell insert, the hydraulic gradient moves upward through capillary action. The uppermost fraction of the germination substrate remains noticeably drier and more aerated than the lower third, forming a dry zone at the soil-air boundary where fungal infection is most frequent.
- Inspect trays to confirm uniform dibble depth and substrate density, as variable compaction distorts capillary lift.
- Flood the benches with tempered water, ideally held at 20 degrees Celsius, to a depth of two to three centimeters over an eight-minute interval.
- Permit capillary uptake for ten to twelve minutes, monitoring the damp line until it rises to within one centimeter of the surface without pooling at the top.
- Rapidly drain the excess solution via high-volume return lines to prevent root-zone hypoxia, diverting the effluent through an inline mechanical disc filter and a closed-loop ultraviolet sterilization reactor before recycling.
- Allow the top layer of substrate to dry sufficiently between irrigation cycles so that the surface displays light coloration before reintroducing moisture.
Biological Inoculants for Root Collar Protection
Even with rigorous sanitation and careful irrigation, total exclusion of pathogens remains difficult in continuous propagation settings. The prophylactic introduction of antagonistic biological agents creates an active biological shield along vulnerable root surfaces. These beneficial organisms protect the root collar through competitive exclusion, digestive balance, and systemic acquired resistance.
The fungal antagonist Trichoderma harzianum (strain T-22 or Rifai) is particularly suited for this purpose. When blended into the potting media at a rate of roughly 100 grams per cubic meter of substrate, Trichoderma colonizes the exterior surfaces of emergent radicles. As the roots expand, the fungal mycelium tracks with them, feeding on sloughed cortical cells and physically blocking Pythium from reaching host tissue. Furthermore, Trichoderma synthesizes chitinases and glucanases that degrade the structural integrity of encroaching pathogenic hyphae.
Bacterial antagonists offer complementary protection under warmer operational regimes. Bacillus amyloliquefaciens strain D747 and Bacillus subtilis produce cyclic lipopeptides, notably iturins and surfactins, which disrupt fungal cell membranes upon contact. Incorporating these bacterial strains via initial soak water creates an inhibitory perimeter around the seed coat during the high-risk germination window.
For operations experiencing recurring soil-borne losses, beneficial actinobacteria like Streptomyces griseoviridis (strain K61) offer prolonged rhizosphere defense. Streptomyces establishes dense colonies on root tissue, secreting broad-spectrum daily routine metabolites that arrest Fusarium mycelial development. These inoculants must be applied proactively during sowing; introducing them after hypocotyl lesions appear yields negligible curative benefit.
Common Mistakes
- Sowing seeds too densely in continuous flats, which traps ambient moisture beneath a closed canopy and ensures rapid root-to-root transmission of fungal hyphae.
- Running bottom heat plates constantly without monitoring core tray temperature, causing warm root systems to transpire aggressively into cold, unconditioned ambient chamber air.
- Reusing polystyrene cell trays without deep sanitization, relying instead on surface dips that fail to reach pathogens embedded within the expanded bead foam.
- Applying overhead irrigation late in the operational photoperiod, leaving wet foliage and saturated collar zones resting in the dark without active transpiration.
- Over-applying biological inoculants alongside synthetic fungicidal drenches, which can neutralize beneficial mycelial networks before they colonize the root system.
Practical Next Steps
To overhaul sanitation and climate protocols within an active closed-cycle chamber, begin with an audit of environmental uniformity. Place calibrated psychrometers at the tray level across multiple vertical shelf tiers to identify microclimatic dead zones where vapor pressure deficit dips below 0.7 kiloPascals. If variance across the chamber exceeds 15% relative humidity, reconfigure circulation fans to establish uniform horizontal airflow before planting valuable seed lots.
Next, evaluate the nursery water delivery infrastructure. If current production relies on overhead mist bars, test conversion to ebb-and-flow trays on a single test rack, or fit fine-mist lines with pressure-compensating check valves to eliminate post-cycle drippage onto center cells. Establish a sanitation schedule requiring total decontamination of all propagation inserts with peracetic acid between germination cycles. If persistent stem collapse continues despite these mechanical interventions, send symptomatic seedlings and intact substrate plugs to a certified agricultural extension laboratory to identify specific pathogens before introducing targeted biological agents or registered chemical controls.